Water Deer - Evolution
Chinese water deer are the only living deer in which males lack antlers, and they sport long, tusk-like upper canines instead. Both traits once looked primitive, as though water deer were a relic of the earliest deer. The evidence now points the other way: most analyses place them within the Capreolinae (the subfamily that includes roe, reindeer, moose and the American deer - see: Taxonomy - True Deer), and they appear to have descended from antlered ancestors that lost their antlers secondarily. This section traces how deer arose, where water deer sit in that story, what the sparse fossil record can and can't tell us, and how genetics has overturned the old view.
Table of contents
The dawn of deer
Deer belong to the artiodactyls, or even-toed ungulates, and the earliest known member of that group is a rabbit-sized mammal called Diacodexis, which inhabited forests of Europe and North America early in the Eocene, some 50 million years ago (mya). These first artiodactyls were small, short-legged creatures that probably fed on leaves and succulent plant material. By the end of the Oligocene, the three suborders we see today can be recognised: the Suina (pigs), the Tylopoda (camels) and the Ruminantia (ruminants including deer, cattle, chevrotains, etc.).
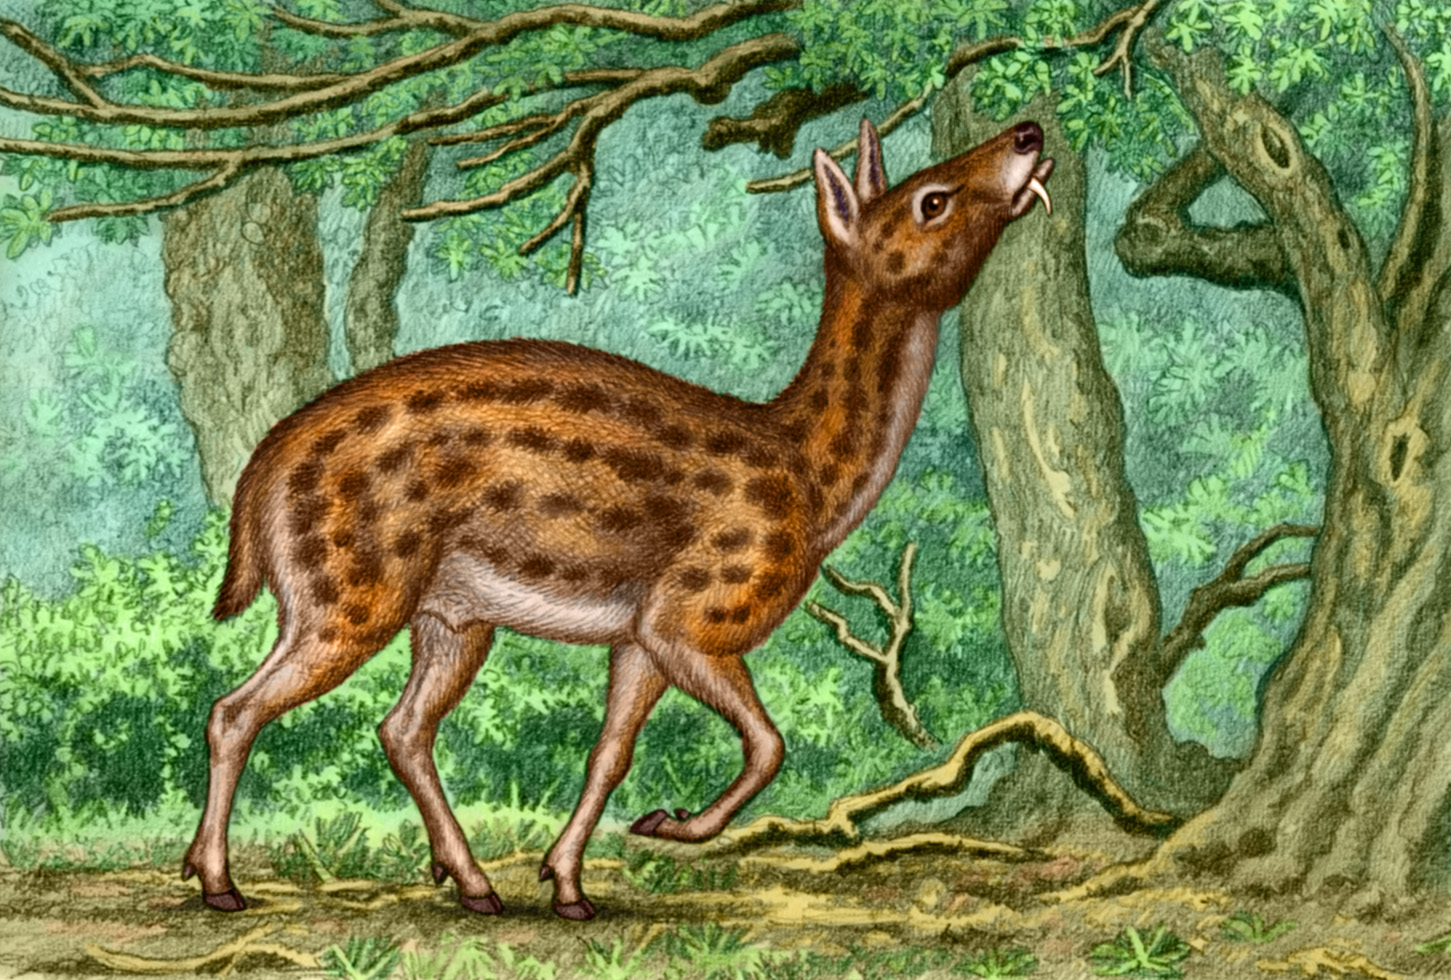
The earliest ruminants appear in the Eocene fossil record, but it was after a widespread mammalian extinction event at the Eocene–Oligocene boundary, around 34 mya, that ruminants similar in appearance to today's duikers (small African antelopes) and chevrotains (small Asian and African "mouse-deer") appear to have diversified. In the same period, we see the development of large canines for use in combat. Deer are believed to have evolved from ruminants of this kind -- small and antlerless, such as the gelocids -- which resembled modern chevrotains. In his 1966 appraisal of cervid evolution, Valerius Geist noted that these early genera were antlerless but possessed large upper canines. Most present-day genera, by contrast, have medium to large antlers and have either lost their upper canines or grow only vestigial ones.
Genetic analysis by Clément Gilbert and colleagues, published in 2006, suggested an Asian origin for the Cervidae (true deer). The oldest deer fossils date from the Early Miocene, around 20 mya, and Gilbert's data indicate that the "crown" group (the last common ancestor of all living deer and its descendants) arose about 10 mya. At the chromosomal level, Ling Huang and colleagues at the Kunming Institute of Zoology in China used chromosome painting in 2006 to show that six chromosomal fissions appear to have transformed the ancestral pecoran karyotype -- the pecorans being the advanced ruminants, including deer, giraffes and cattle -- of 58 chromosomes (2n) into the ancestral cervid karyotype of 70. Water deer have retained that number, as have roe (Capreolus), grey brocket (Mazama gouazoubira) and the white-tailed and mule deer (Odocoileus), while other cervids have the same or commonly fewer (Cervus have 60–68, for example). In their 1988 publication on deer genetics, Zongren Wang and Ruofu Du suggested that chromosome evolution in the Cervidae has been towards fewer chromosomes, indicating that 70 probably represents the ancestral state. That makes water deer chromosomally conservative, but retaining an ancestral trait isn't evidence that a lineage branched off early, so it can't tell us where they sit in the family tree.
So where do water deer fit, and when did they branch off? The Capreolinae subfamily (roe, reindeer, moose and the American deer, with which water deer are now generally grouped) emerged, according to Gilbert and his team, in Central Asia at the Miocene/Pliocene boundary (~5 mya) as Procapreolus and diversified there before migrating into what is now North America.*
In their 2004 analysis of Old World deer phylogeny, Christian Pitra and colleagues pointed out that while the Asian genus Procapreolus is considered ancestral to Capreolus, it remains unclear (and in their view, unlikely) whether Procapreolus latifrons is also ancestral to Hydropotes. This species inhabited the Late Miocene–Early Pliocene forests of Asia some 5.5 mya and appears to be the ancestor of modern roe. Indeed, in a 1998 paper to the Proceedings of the Royal Society of London, a team led by Ettore Randi at the Istituto Nazionale per la Fauna Selvatica in Italy calculated, based on cytochrome b nucleotide sequences, that the lineages for modern water and roe deer diverged well before P. latifrons appeared on the scene, in the Late Miocene about 11 mya. That estimate used the early "strict" molecular clock, however, which is now known to be less accurate than the modern "relaxed" clock used by Gilbert and subsequent authors. These more recent data suggest the split occurred much more recently, Hydropotes diverging from Capreolus 5–6 mya, which narrows the gap to P. latifrons considerably.
--
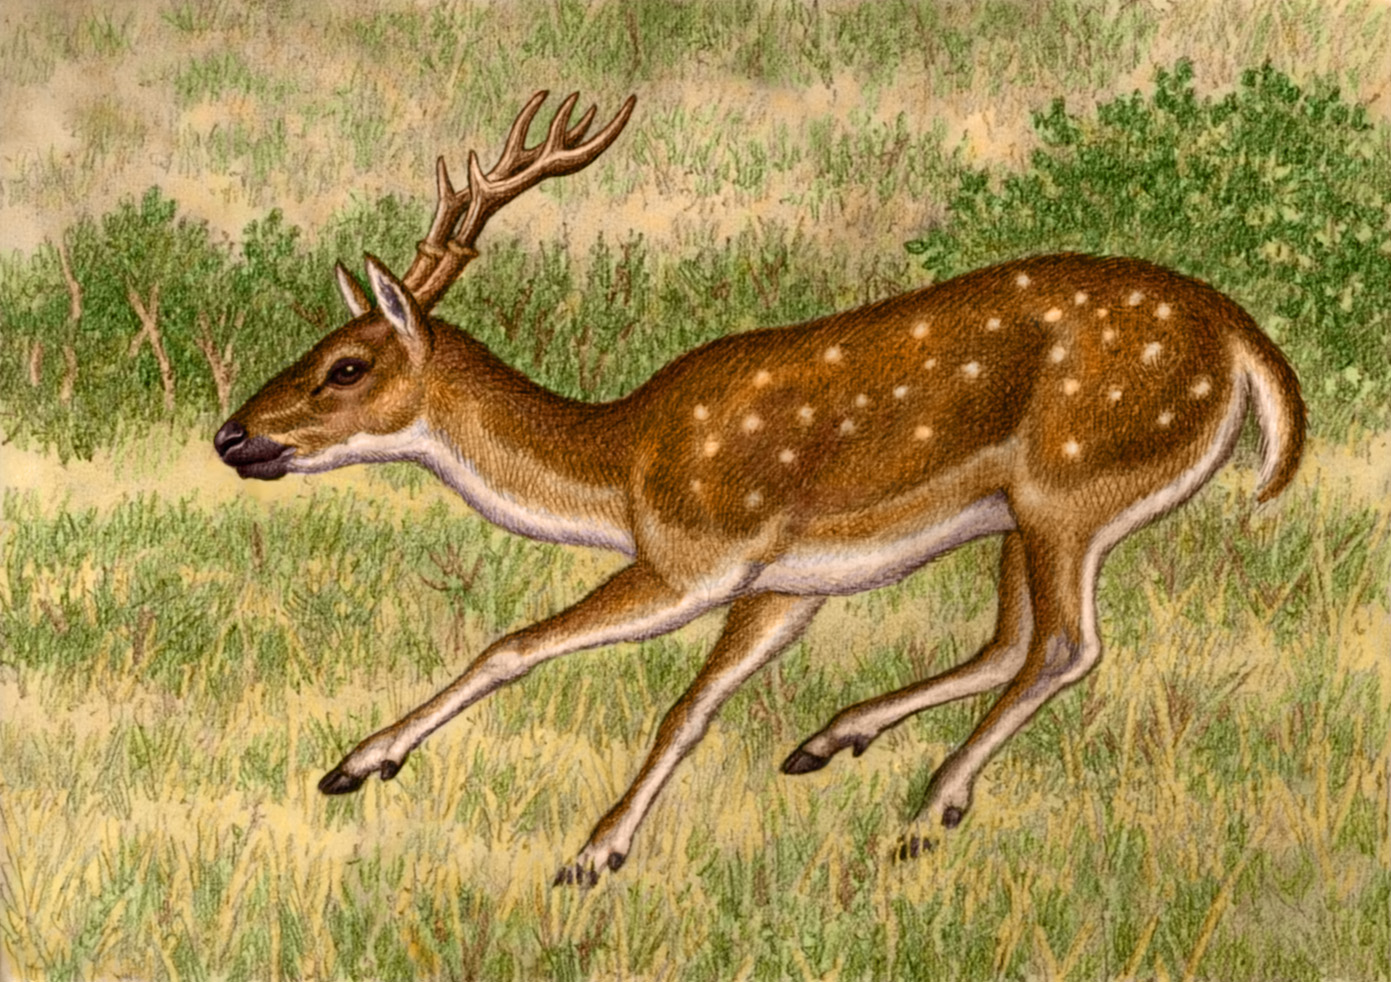
That tells us roughly when water deer split from the roe line, but not what they split from. During the 1960s and '70s -- see the work of Denise Sigogneau (1968) and William Hamilton (1973), for example -- several authors suggested Dremotherium, from the Late Oligocene of Europe and Asia (~25 mya), as the ancestor of both musk and water deer. This is perhaps understandable, given they share large canines and lack antlers, but both the difference in soft tissue anatomy between the species and molecular data cast some doubt on it. In 2003, Alexandre Hassanin and Emmanuel Douzery confirmed, through genetic analysis, that the Moschidae pair with the Bovidae and not the Cervidae, as was originally thought, and the Cervidae lineage is thought to have separated from them around 27–28 mya, before Dremotherium appears in the fossil record. Any ancestor shared by musk and water deer would have to predate that split, so Dremotherium can't be it, and musk deer aren't close relatives of water deer after all.
If Dremotherium isn't the answer, can the fossils of water deer themselves help? Sadly, there's not much to go on. Yeong-Seok Jo, John Baccus and John Koprowski note, in their 2018 Mammals of Korea, that the water deer was present in Korea during the first half of the Quaternary, suggesting they've been in Asia two million years or so, though the authors don't cite a source. I'm currently not aware of any fossil evidence of water deer from Korea but would be interested to hear from any readers who are.
Wei Dong, in her chapter in the 1993 Deer of China compendium, listed the oldest fossil of Hydropotes from the Middle Pleistocene of northern China (800,000–120,000 years ago). I think this is from Zhoukoudian (historically, the Sinanthropus Site at Chouk'outien), although the author doesn't specify. Likewise, in his 1972 paper to the Journal of Mammalogy, Peter Brokx wrote that the water deer was "not known from before the Pleistocene". Brokx cited George Simpson's 1945 work on the principles of mammalian classification for this, although Simpson listed the water deer only as "recent", which going by his scheme is Holocene (i.e., the current geological epoch, which began around 11,700 years ago).
Antlers answered?
A curious feature of this species, and one that sets it apart from all other members of the deer family, is that the males lack antlers. Bony structures emanating from specialised outgrowths on the frontal bone of the skull called pedicles, antlers are more than just ornaments evincing fitness; they're an integral component in securing mating opportunities in a family where males must fight one another for access to females (see Antler Development). By the Middle Pleistocene when water deer seem to have evolved, this headgear had been a feature of the deer family for many millions of years. Consequently, their absence here raises an interesting evolutionary question: does the water deer represent the primitive form (ancestral phenotype) of deer, or is antler loss an autapomorphy (i.e., derived)? In other words, did the first deer to walk the earth look like a water deer, with antlers evolving later in other lineages, or did it sport antlers that were subsequently lost somewhere along the water deer's ancestral line – a secondary loss? The weight of evidence now favours the latter, though it took a while to get there.
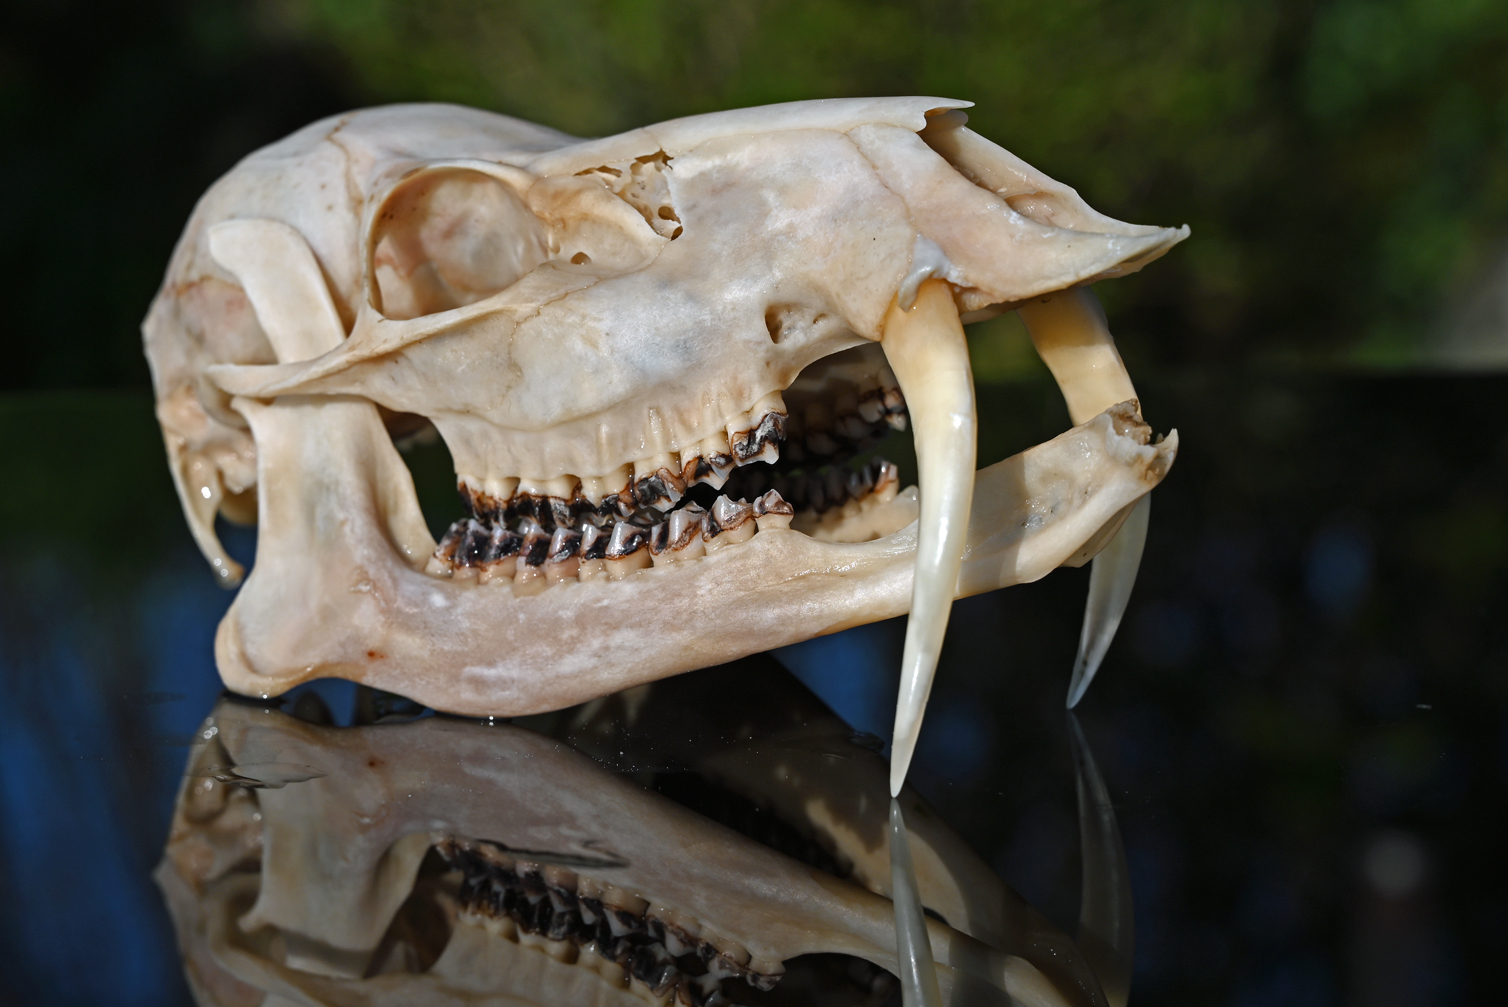
In their deer classification scheme, published in 1987, zoologists Paul Groves and Peter Grubb considered water deer to be the sister group to all other cervids. In other words, they viewed both the presence of well-developed canines and the absence of antlers as primitive traits. On this interpretation, the earliest deer had tusks, and as antlers evolved most species lost their canines in favour of headgear. In 1998, however, renowned deer evolutionary biologist Valerius Geist argued that the morphology and life history traits of water deer don't appear to match what we know about the primitive tropical deer from which modern cervids descended. Geist championed an idea first proposed by Russian zoologist Konstantin Flerov in 1950: that the lack of antlers in Hydropotes is not a primitive retention but a secondary loss. Randi and his colleagues, in their 1998 paper, arrived at the same conclusion, this time on the basis of molecular evidence, writing:
"Contrasting with current taxonomy, Hydropotes is not the sister group of all the antlered deers, but it is nested within the Capreolinae. Therefore, Hydropotes lost the antlers secondarily."
Corroboration followed in 2003, when Ming Li and her team published a cytochrome b dataset in Acta Theriologica that supported the emergence of water deer from an antlered ancestral line. Two years later, in his 2005 revision, Grubb updated his own earlier stance, placing water deer as a sister subfamily to the Capreolinae – an arrangement that, while not widely adopted, more closely reflected the growing consensus that antler loss in this species is indeed secondary.
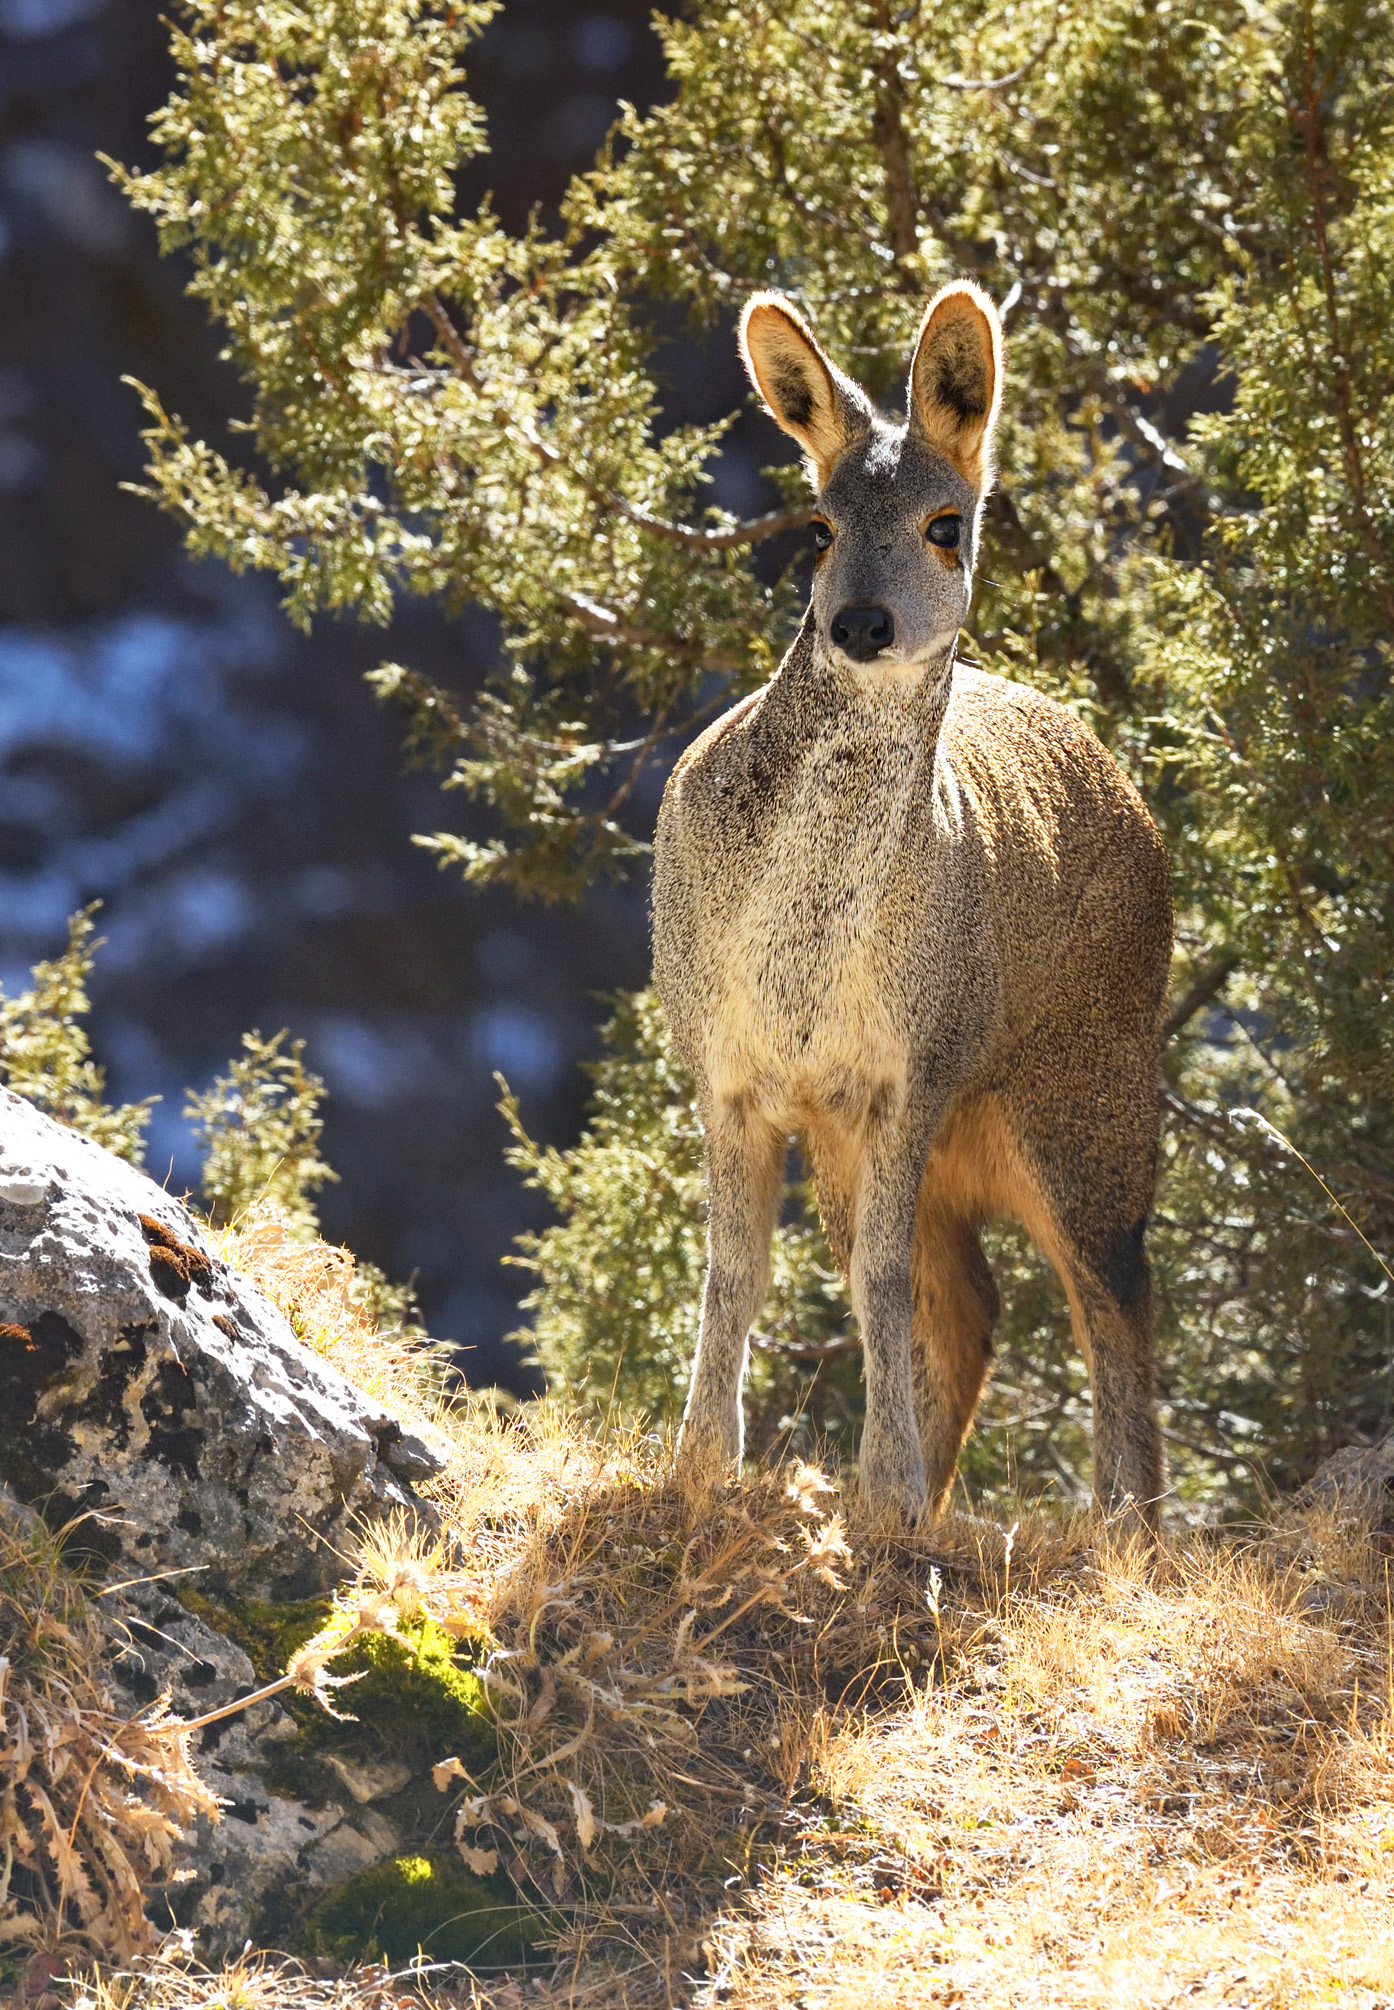
More recently, a 2026 genomic study by Zhenyu Zhong, Lisen Li and colleagues, published in Zoological Research, sequenced six deer genomes, including the water deer's, and compared the genes of antlered and antlerless species. They found 40 genes completely lost in water deer and a further 188 under relaxed selection. In a nutshell, the pressure that once preserved those genes has slackened, so mutations that damage them are no longer being weeded out. Six of the lost genes, including one called RXFP2, are highly expressed in the antler buds of sika deer (Cervus nippon), which is what we'd expect if water deer have lost working copies of genes their antlered relatives use to grow antlers. The authors also highlight the loss of ZNF675, a gene that restrains bone resorption, suggesting a link to the unusual skeletal physiology of antlered deer, which draw calcium from the rest of the skeleton while their antlers grow.
RXFP2 is of particular interest and, citing earlier work, the authors noted that the same gene appears to have failed independently in musk deer (Moschus), the only other living group of pecorans to have lost their headgear, and point out that their own data corroborate the pattern. As we saw above, musk deer aren't close relatives of water deer, so this looks like a genuinely independent loss. Two separate lineages losing their headgear and the same gene breaking in both is suggestive of a real role in antler development, although it doesn't prove one. And since the 188 relaxed genes are decaying rather than already gone, I suspect the process is still under way – but that's my interpretation of the paper, not a claim the authors make.
Putting these strands together, the case for secondary loss rests chiefly on where water deer sit in the family tree, not on the fossils. Antlered cervids such as Procervulus are known from the Early Miocene, well before the Capreolinae diversified. If Hydropotes is nested within the antlered deer -- as Randi and later molecular studies indicate, and as Grubb's 2005 arrangement also implies, with water deer as sister to the Capreolinae -- the simplest explanation is that its ancestors had antlers. To assume otherwise, antlers would have had to evolve independently in several different lineages. The ruminants ancestral to deer were antlerless and tusked, which is why Groves and Grubb's conclusion was reasonable on morphology alone, but their placement of water deer as sister to all other deer is the one thing the molecular data have consistently overturned.
The genomic evidence points the same way. A gene can only degrade into a pseudogene if it was once functional; so, the remnants of antler-development genes in water deer are the signature of something lost, not something that never evolved. As for the canines, the simplest interpretation is that they were retained from the antlerless ancestors of all deer and, in water deer, became the primary weapon once antlers were gone. Whether these canines were actively enlarged beyond the ancestral condition, which seems likely to me based on what we see in more ancestral lineages within the artiodactyls, is a separate question that remains untested.
References
Brokx, P.A. (1972). The superior canines of Odocoileus and other deer. Journal of Mammalogy. 53: 359-366.
Dong, W. (1993). A morphological analysis of cheek teeth of Eurasian Pliocene cervids. In: Ohtaishi, N. & Sheng, H-I. (eds). Deer of China. Elsevier Science Publishers. pp. 65-72.
Flerov, K.K. (1950). Morphology and ecology of cervines in process evolution. Material of the Quaternary Period of the U.S.S.R., Academy of Sciences of the U.S.S.R., Moscow. Part 2, pp. 50-69. [In Russian]
Geist, V. (1966). The evolution of horn-like organs. Behavior. 27: 175-214.
Geist, V. (1998). Deer of the World: Their Evolution, Behaviour, and Ecology. Stackpole Books, London.
Gilbert, C. et al. (2006). Mitochondrial and nuclear phylogenies of Cervidae (Mammalia, Ruminantia): Systematics, morphology, and biogeography. Molecular Phylogenetics and Evolution. 40: 101-117.
Groves, C.P. & Grubb, P. (1987). Relationships of living deer. pp. 21-59. In: Wemmer, C.M. (ed.) Biology and Management of the Cervidae. Research Symposia of the National Zoological Park. Smithsonian Institution Press, Washington.
Grubb, P. (2005). Order Artiodactyla. In: Wilson, D.E. & Reeder, D.M. (eds). Mammal Species of the World: A taxonomic and geographic reference (Vol 12). Johns Hopkins University Press, Baltimore, Maryland. p. 637-722.
Hamilton, W.R. (1973). The Lower Miocene ruminants of Gebel Zelten, Libya. Bulletin of the British Museum (Natural History) Geology. 21: 75-150.
Hassanin, A. & Douzery, E.J.P. (2003). Molecular and morphological phylogenies of the Runinantia and the alternative position of the Moschidae. Systematic Biology. 52: 206-228.
Huang, L. et al. (2006). Phylogenomics of several deer species revealed by comparative chromosome painting with Chinese muntjac paints. Genetica. 127: 25-33.
Jo, Y-S. et al. (2018). Mammals of Korea. Life Science Publishing Co., Seoul.
Li, M. et al. (2003). Phylogenetic relationships among deer in China derived from mitochondrial DNA cytochrome b sequences. Acta Theriologica. 48: 207-219.
Pitra, C. et al. (2004). Evolution and phylogeny of old world deer. Molecular Phylogenetics and Evolution. 33: 880-895.
Randi, E. et al. (1998). New phylogenetic perspectives on the Cervidae (Artiodactyla) are provided by the mitochondrial cytochrome b gene. Proceedings of the Royal Society o London. 265B: 793-801.
Sigognerau, D. (1968). Le genre Dremotherium (Cervoidea). Anatomie du crâne, denture et moulage endocrânien. Annales de Paléontologie (Vertébrés). 54: 39-64.
Simpson, G.G. (1945). The principles of classification and a classification of mammals. Bulletin of the American Museum of Natural History. 85: 1-350.
Wang, Z. & Du, R. (1988). 鹿的核型与染色体进化 (The Karyotype and Chromosome Evolution of Deer). Science Publish House, Bejing. [In Chinese]
Zhong, Z et al. (2026). Phylogenomic analysis of Cervidae provides insights into antler origin and evolution. Zoological Research. 47: 289-302.